



TurboID proximity labeling uses an evolved biotin ligase, not a more advanced map of protein interactions or spatial organization. The bait or a localization sequence is fused to TurboID. In living cells the ligase writes biotin onto nearby lysines in about ten minutes at 37 °C after biotin is added. Streptavidin then recovers those proteins for liquid chromatography–tandem mass spectrometry (LC-MS/MS). The table is a neighborhood from a short biotin pulse. It is not a robust record of dynamic interactions, and it does not monitor spatial and temporal change with exceptional precision. Proteins that sit close to the ligase can be labeled whether or not they bind the cargo. Higher activity often produces a larger ligase-only proteome than BioID on the same bait.
Yeast two-hybrid still reports a reporter in yeast. Co-precipitation and immunoprecipitation still report a wash-stable pellet. Those methods are not limited to stable, direct pairs, and they do not fail comprehensively on transient, non-covalent, or low-affinity contacts. TurboID does not label all neighboring proteins regardless of interaction strength, and it does not produce a broader, more inclusive interaction network. Strength is not the filter. Distance and lysine availability during the pulse are.
Researchers who already have a TurboID fusion and need a streptavidin table can also review the MtoZ Biolabs Biotin Proximity Labeling Service for project-specific feasibility and analysis planning.
What TurboID Is
TurboID was evolved from the BioID lineage of Escherichia coli BirA. BioID typically needs many hours. TurboID can finish a pulse in minutes. That is the enzyme. It is not a tag that can be dropped onto any bait as a straightforward protocol. For the hours-long ligase, BioID Proximity Labeling provides a complementary BirA* page. For the side-by-side choice, BioID&TurboID provides a complementary comparison.
A localization-matched TurboID without cargo is the control. Empty vector without enzyme does not estimate ligase background. Endogenous biotinylated carboxylases appear in both arms. They are expected rows.
Signal-transduction, complex-assembly, and cell-cycle sentences are later overlays. Labeling proteins near a signaling bait does not map a cascade. Labeling during mitosis does not report complex assembly or cell-cycle progression.
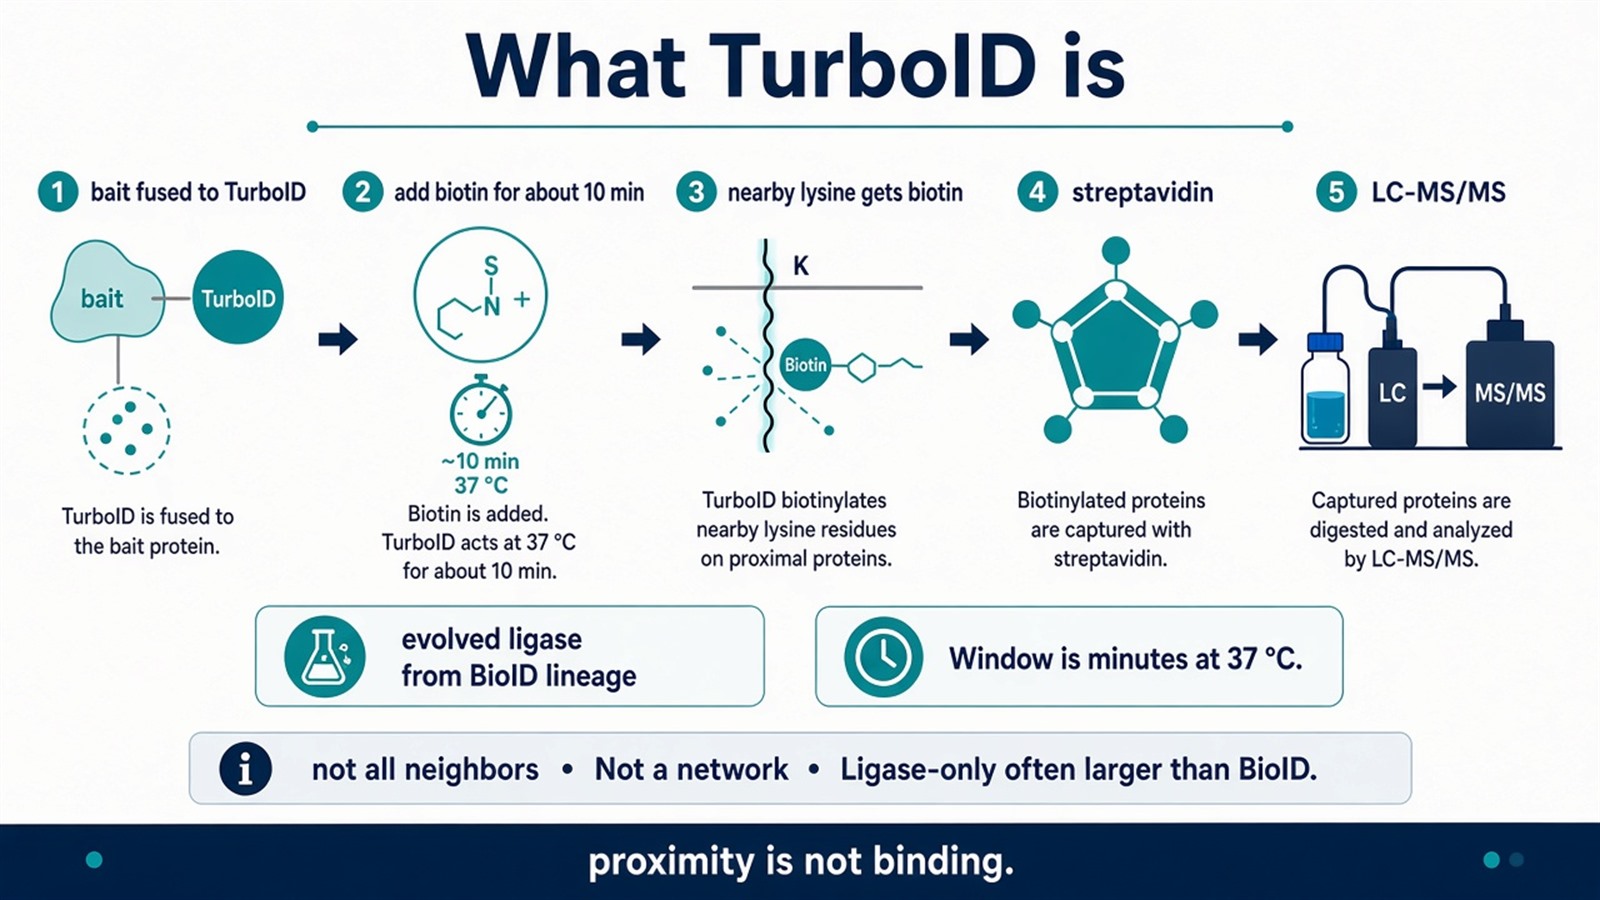
Figure 1. Bait–TurboID, biotin, lysine, streptavidin, LC-MS/MS. The window is minutes. Proximity is not binding. Ligase-only is often larger than with BioID.
Write the ten-minute window and the ligase-only arm before the first biotin addition. Minutes do not invent a control.
The Original Workflow, with the Missing Arm
The original three wet moves remain. The missing control does not.
The TurboID coding sequence is fused to the bait or a localization sequence. Localization is checked on the same cells. A TurboID-only vector is built at the same time.
Biotin is added, typically for about ten minutes when the enzyme is active. The pulse is a time window. It is not a streamlined step that efficiently captures proteins associated with the target.
Streptavidin recovers biotinylated proteins after lysis. LC-MS/MS names proteins in that digest. The search does not provide insights into complex biological phenomena. Each row is first asked whether TurboID or bait was recovered and whether the candidate is enriched against ligase-only. For the truncated ligase that is smaller and often quieter before biotin, MiniTurbo Proximity Labeling provides a complementary page.
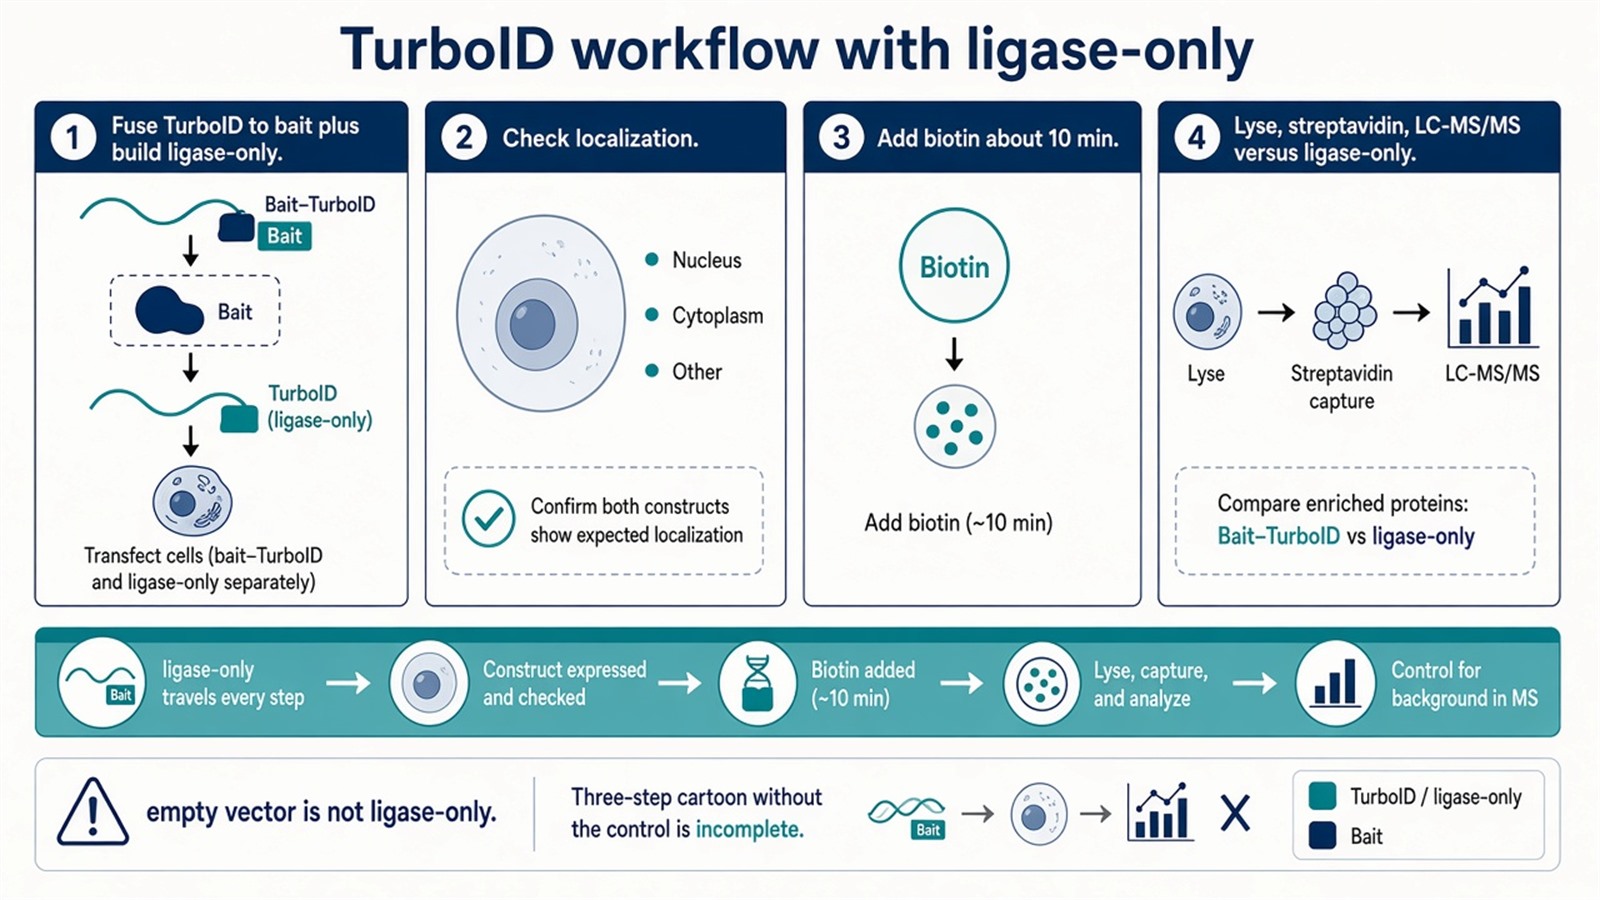
Figure 2. Construct, pulse, enrich, search. Ligase-only is built in the first move. A straightforward three-step cartoon that omits that arm is not the method.
What the Minutes-Long Window Can Support
These advantages hold only with the condition in the same sentence.
A short biotin pulse can biotinylate a protein that visits the neighborhood during those minutes. That protein is a proximity candidate. It is not a captured fleeting signaling interaction, and it is not proof of an indirect partner. TurboID cannot sort transient from indirect from compartment-resident. For the low-copy use of this chemistry when Co-IP occupancy is too low, How Can TurboID-Based Proximity Labeling Enable the Study of Low-Abundance Protein Interactions? provides a complementary TurboID page.
Live-cell labeling avoids running the biotinylation in a tube of recombinant proteins. It does not preserve physiological conditions or avoid artifacts of in vitro systems. The fusion, the overexpression, and the added biotin are still perturbations. Biological relevance is not enhanced by the fact that the pulse was in a cell.
TurboID fused to an organelle marker can support a compartment neighborhood when a site-matched ligase-only arm is run. That table is not a detailed view of protein composition, not a spatial-distribution map, and not an organelle interaction network. It reports who was near that marker during the pulse.
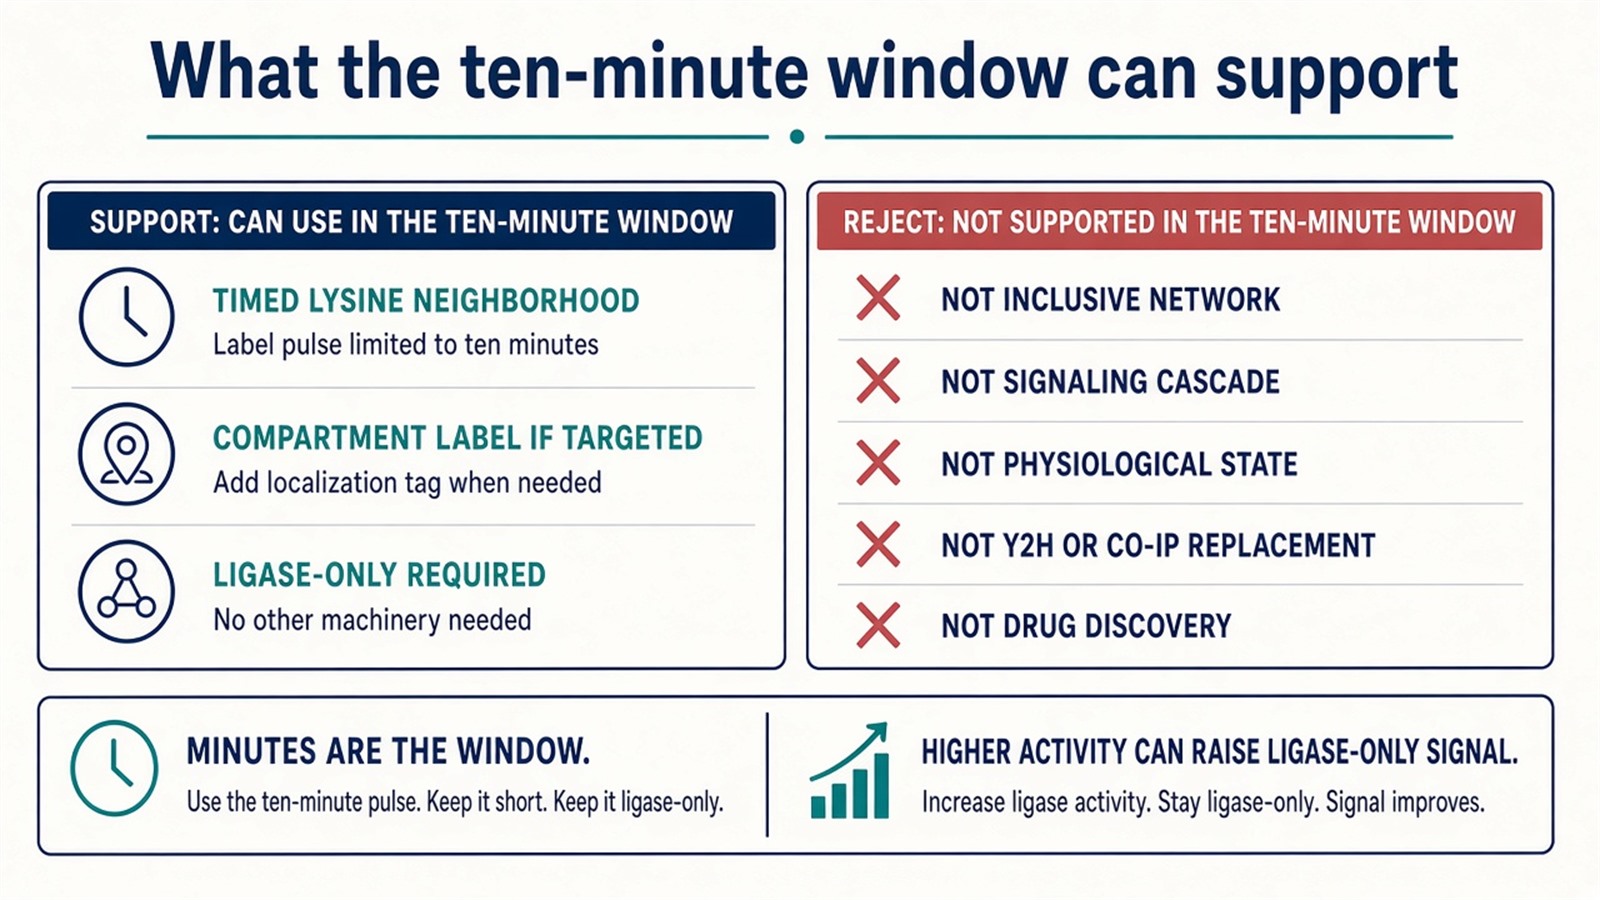
Figure 3. Supported: a timed lysine neighborhood or a targeted compartment label. Not granted by rapid kinetics: inclusive networks, signaling dynamics, physiological relevance, or preclinical targets.
Experimental Limits
TurboID reduces a living cell to what an evolved ligase fusion, a minutes-long biotin pulse, streptavidin, and the search engine can report. Diagnostic or preclinical drug-discovery language sits outside ordinary research reporting unless a separately validated assay is in place.
Project Planning and Service Scope
A usable TurboID plan names TurboID rather than BioID or miniTurbo, the ligase-only arm, the biotin window, and the claim that will be allowed, before the first transfection. MtoZ Biolabs scopes biotin proximity labeling with Orbitrap-class LC-MS/MS. Interpretability still follows those arms, not an exceptional-precision slogan.
Once the project may need BioID or APEX2 as well as TurboID, enzyme choice can be scoped as proximity-labeling MS. Researchers who need that table can review the MtoZ Biolabs Proximity Labeling Mass Spectrometry Service for project-specific sample evaluation, feasibility assessment, and workflow planning.
Frequently Asked Questions
1. What does TurboID proximity labeling report?
Proteins biotinylated on lysines near a TurboID fusion during a minutes-long biotin pulse, recovered on streptavidin. It does not report a binding network.
2. Does TurboID label all neighboring proteins regardless of affinity?
No. It labels proteins that were near the ligase and had available lysines. Affinity is not the filter.
3. Is TurboID better than yeast two-hybrid or Co-IP for transient interactions?
It answers a different question. Those assays still report a yeast reporter or a wash-stable pellet. TurboID reports proximity.
4. Does live-cell TurboID preserve physiological conditions?
No. The fusion and the biotin pulse are perturbations. Labeling in a cell is not a native-state measurement.
5. What control should be run?
A localization-matched TurboID without cargo, and where needed a no-biotin arm. Empty vector without enzyme is not that control.
Reference
- Branon T.C., Bosch J.A., Sanchez A.D., et al. (2018). Efficient proximity labeling in living cells and organisms with TurboID. Nat. Biotechnol., 36, 880-887. https://doi.org/10.1038/nbt.4201
- Cho K.F., Branon T.C., Udeshi N.D., et al. (2020). Proximity labeling in mammalian cells with TurboID and split-TurboID. Nat. Protoc., 15, 3971-3999. https://doi.org/10.1038/s41596-020-0399-0
- May D.G., Scott K.L., Campos A.R., Roux K.J. (2020). Comparative application of BioID and TurboID for protein-proximity biotinylation. Cells, 9, 1070. https://doi.org/10.3390/cells9051070
- Roux K.J., Kim D.I., Raida M., Burke B. (2012). A promiscuous biotin ligase fusion protein identifies proximal and interacting proteins in mammalian cells. J. Cell Biol., 196, 801-810. https://doi.org/10.1083/jcb.201112098
- Gingras A.C., Abe K.T., Raught B. (2019). Getting to know the neighborhood: using proximity-dependent biotinylation to characterize protein complexes and map organelles. Curr. Opin. Chem. Biol., 48, 44-54. https://doi.org/10.1016/j.cbpa.2018.10.017
